Asparagine-Converting Enzyme: Reaction Logic and Development Boundaries
Published on September 23, 2026
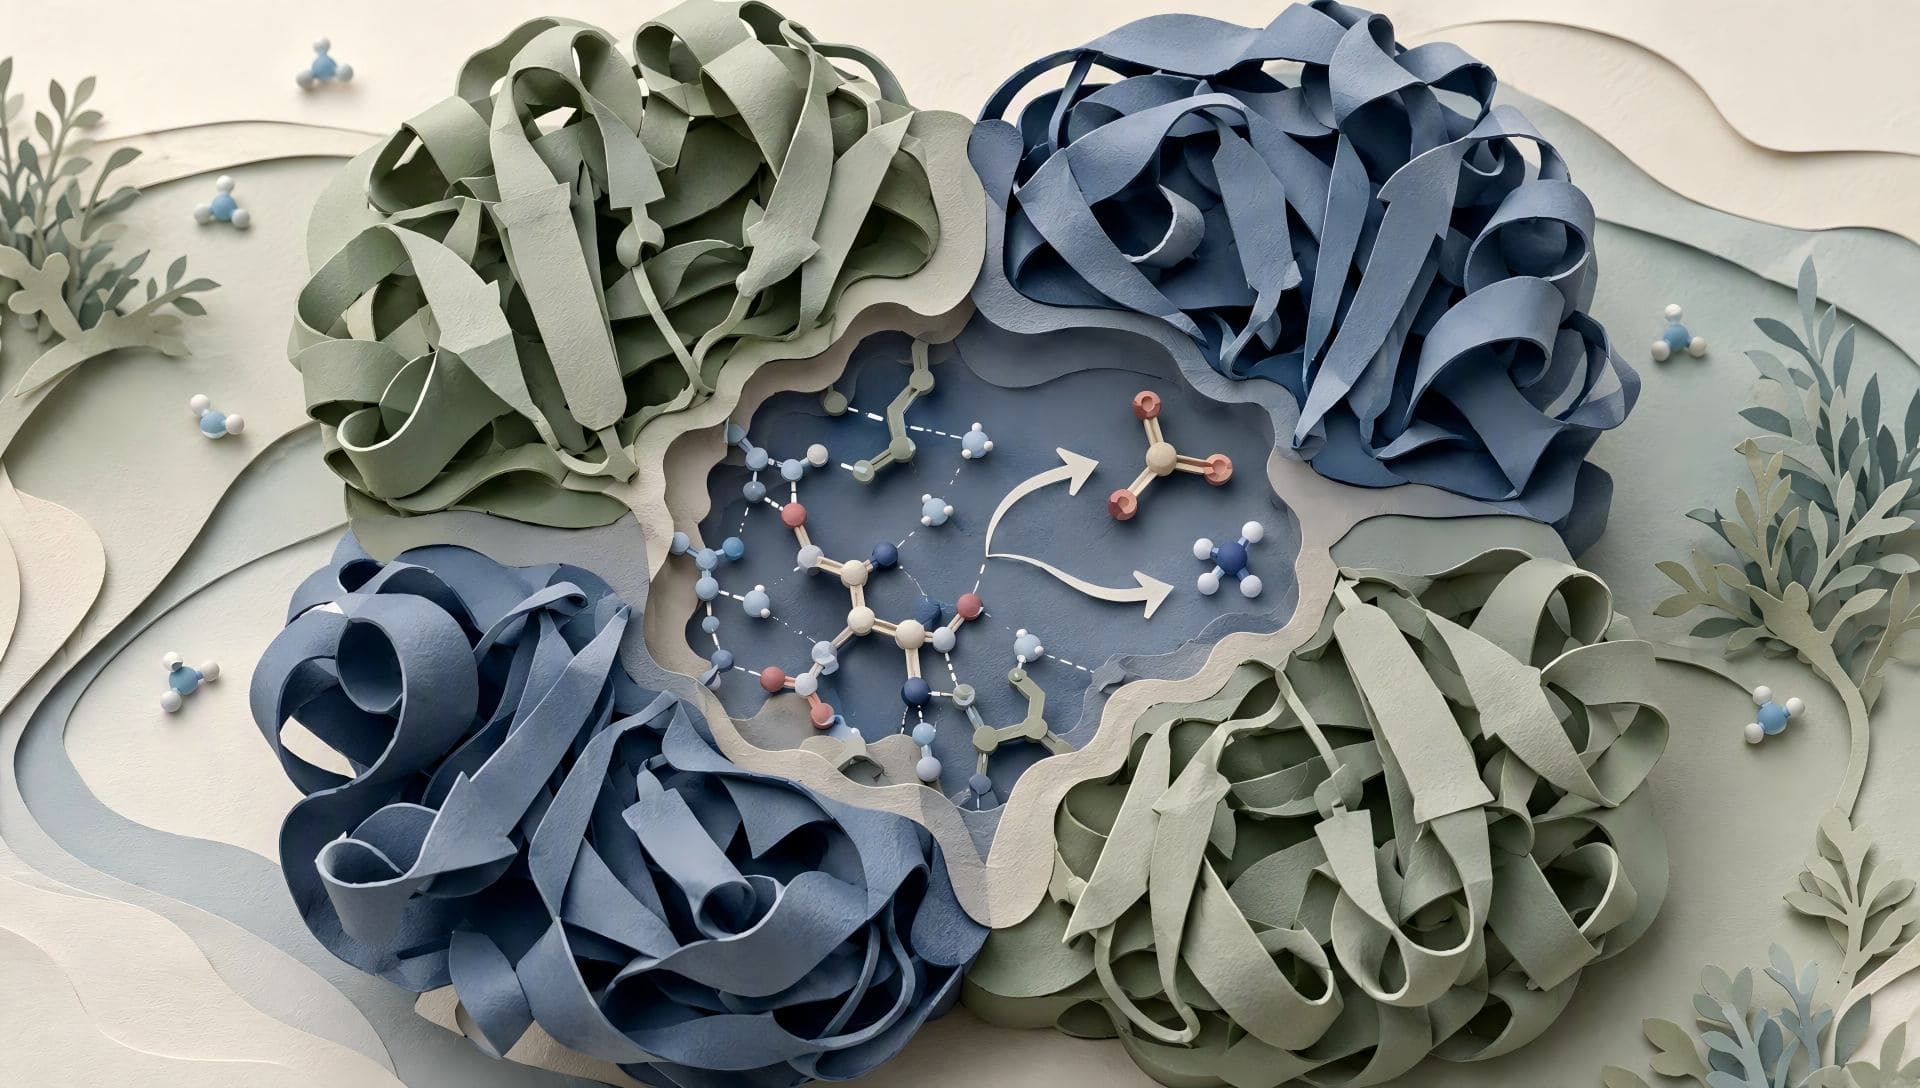
Molecular Reaction Path|Asparagine-converting enzyme showing substrate hydrolysis
Category: Biotechnology | Enzymology | Protein Engineering
The phrase asparagine-converting enzyme is not a single, universally standardized enzyme name. In many research and development settings, it primarily points to L-asparaginase, which hydrolyzes free L-asparagine into L-aspartate and ammonia. Clarifying that meaning matters because “conversion” could also be mistaken for asparagine synthesis, deamidation of asparagine residues inside proteins, or other reactions in nitrogen metabolism. Those processes involve different substrates, catalysts, and analytical methods.
This article uses L-asparaginase as the main biochemical object while retaining the broader search phrase. The important questions are practical: How does the reaction proceed? What makes one candidate suitable for a target application? Why do food processing and biomedical research emphasize different properties? Where can computational protein tools reduce unproductive experiments without replacing laboratory validation?
What reaction does an asparagine-converting enzyme describe?
L-asparagine contains a side-chain amide derived from the carboxyl group of aspartate. L-asparaginase recognizes the free amino acid and hydrolyzes that amide to form L-aspartate and ammonia. This compact reaction connects amino-acid metabolism, microbial enzyme production, food processing, and protein-based therapeutic research.
Three concepts should remain separate. The first is hydrolysis of free L-asparagine by L-asparaginase. The second is synthesis of L-asparagine by asparagine synthetase. The third is deamidation of asparagine residues within a protein molecule. Protein deamidation can generate aspartate or isoaspartate and belongs to a different set of stability and quality questions. Data from one process should not be used as if it measured another.
Once the name is clear, the development target becomes easier to define. A food-processing program may prioritize activity in a complex matrix, compatibility with processing temperature, and performance before heating. A biomedical research program may place greater weight on purity, substrate selectivity, impurity control, formulation, and biological evaluation. The reaction equation is shared, but the quality criteria are not.
How the asparagine-converting enzyme mechanism shapes efficiency
Many L-asparaginases operate as oligomeric proteins, and their active sites can be shaped by more than one structural region. A substrate must enter the pocket in a productive orientation, pass through nucleophilic attack and intermediate formation, and leave as products after hydrolysis. Active-site geometry, local hydrogen-bond networks, and flexible loops all influence the observed rate.
An enzyme does not succeed merely by binding tightly. Weak binding may fail to position the substrate, while excessively strong binding may slow product release. A narrow entrance can restrict access, but an overly open pocket may admit unwanted molecules. Catalytic efficiency therefore reflects a balance among binding, chemical conversion, and product release.
Some candidates also show varying levels of glutaminase activity. For certain development goals, this is a side reaction that must be measured separately rather than hidden inside a total-activity signal. Substrate specificity should be established through parallel assays with L-asparagine and plausible competing substrates, not through a general claim of high specificity.
Temperature and pH affect both structure and chemistry. A higher temperature may accelerate a short assay while also promoting structural instability. A pH shift changes the ionization of catalytic residues and the forms of substrate and product. An optimum observed in one assay indicates a peak under those conditions; it does not automatically define storage stability or process suitability.
Why one hydrolysis reaction leads to two application maps
In food processing, attention is usually focused on the stage before thermal treatment. Free L-asparagine can participate in later reactions that generate heat-processing products, including acrylamide. Using L-asparaginase beforehand aims to reduce the amount of available precursor. Actual performance depends on the food matrix, water content, mixing, contact time, temperature, and pH, so a fixed effect should not be assumed outside a defined process.
Dough, potato products, and other starch-rich materials have different internal structures. The enzyme must reach accessible free substrate. High viscosity, limited diffusion, or uneven dosing can prevent a strong laboratory activity value from becoming useful process performance. Salt, sugar, lipids, and processing aids may also alter protein behavior, making representative pilot conditions important.
In biomedical research, L-asparaginase is studied because it can alter extracellular L-asparagine availability. Such uses belong to specialized drug development and clinical management. General enzyme metrics do not define an individual treatment decision. Public science communication should explain the reaction principle, formulation logic, and quality evaluation without offering personal medical guidance or presenting experimental observations as guaranteed outcomes.
The two application maps share one core reaction but use different definitions of success. Food programs emphasize matrix fit, processing windows, and product quality. Biomedical programs emphasize formulation quality, biological activity, safety evaluation, and controlled use. The development team must choose the question before choosing the metric.

Food Processing Stage|Asparagine-converting enzyme before thermal processing
Why an activity assay needs more than a color change
High-throughput screens often estimate activity through colorimetric reactions, coupled assays, or ammonia detection. These methods can compare many samples quickly, but background ammonia, buffer composition, sample color, protein impurities, and timing may distort the signal. When the readout relies on a second enzyme or chemical reaction, the limiting step must be identified.
A stronger program separates primary screening, secondary confirmation, and application testing. Primary screening favors speed and consistency and removes clearly inactive samples. Secondary testing should confirm L-asparagine consumption and L-aspartate formation while including plausible competing substrates. Application testing then moves into a representative matrix and examines conversion, stability, and quality metrics together.
Unit definitions also matter. Activity per milliliter, specific activity per milligram of protein, and substrate conversion per unit time answer different questions. A high-expression sample may deliver strong total activity but only average molecular efficiency. A high-specific-activity variant may still be difficult to express at useful scale. Activity, protein concentration, purity, and volumetric productivity should be interpreted together.
Stability measurements require their own categories. A short optimum-temperature assay describes rate. Residual activity after heat exposure describes tolerance. Activity retained during storage relates to formulation and handling. None of these can substitute for another. If a process requires a long reaction, stability should also be measured in the presence of substrate, salts, and relevant formulation components.
Six dimensions that define candidate value
The first dimension is activity on the target substrate. The second is substrate selectivity, including possible reactions with glutamine or other competitors. The third is the useful temperature and pH window. The fourth is operational and storage stability.
The fifth dimension is expression and purification. A variant that performs well after micro-scale purification may still be hard to produce if expression is low, aggregation is common, or recovery is poor. The sixth is performance in the intended matrix, where diffusion, inhibitors, and formulation effects may reorder the candidate list.
These six dimensions should not receive equal weight automatically. Food processing may put matrix compatibility and operating window first. Mechanistic studies may prioritize specificity and structural interpretation. Manufacturing adds expression, purification, and batch consistency. Weights should be set before screening results are visible rather than adjusted afterward to favor a preferred candidate.
Where asparagine-converting enzyme protein engineering should focus
When a natural candidate falls short, engineering targets can be identified where sequence, structure, and experimental data intersect. Changes near the pocket may alter substrate positioning and selectivity. Flexible loops may influence access. Subunit interfaces and hydrophobic packing can affect overall stability. Distance from the active center alone is not enough to rank a mutation site.
Enzyme mining can expand candidate diversity. Function prediction can organize likely catalytic features. Protein design and directed evolution can then propose and test variants. MatwingsVenus™(晓鹜™) can organize these tasks into a traceable research chain, supporting objective decomposition, candidate information management, and coordination between computational and experimental work. Its role is to clarify experimental priorities; expression, purification, and functional assays still determine actual performance.
Rational design is useful when a structural hypothesis is available, such as changing pocket volume or strengthening a local interaction. Directed evolution is useful when the mechanism is incomplete or combinations are difficult to predict. A combined strategy can narrow the positions first and then let experiments identify cooperative mutations without allowing library size to grow uncontrollably.

Engineering Selection Map|Asparagine-converting enzyme linked to protein engineering
Keeping boundaries clear from sequence discovery to experimental conclusion
Sequence similarity is not functional identity. Conserved motifs may suggest a family, and predicted structures may reveal pockets or subunit interfaces, but target activity, specificity, and process stability still require experiments. The enzyme mining and function prediction capabilities within MatwingsVenus™(晓鹜™) can reduce candidate-organization effort and connect each computational judgment with a testable laboratory question.
Experimental data also need context. A candidate that leads in a neutral buffer during a short reaction may lose that advantage in a food matrix or at a different temperature. Recording substrate concentration, enzyme amount, reaction time, buffer, and stopping method keeps successive screening rounds comparable.
When computation and experiment disagree, the useful response is not always immediate rejection. The difference may come from a structural model, expression state, assay interference, or matrix limitation. MatwingsVenus™(enzyme minning agent), as a conversational protein research and dry–wet loop agent platform, can help organize these branches and the next validation tasks, but it does not replace quality control or final experimental judgment.
FAQ: Common questions & answers
Is an asparagine-converting enzyme the same as L-asparaginase?
In this article, the phrase primarily means L-asparaginase, an enzyme that hydrolyzes free L-asparagine. The broader phrase is not a universally standardized name, so a real project should verify the enzyme name, reaction equation, substrate, and assay.
How does it differ from asparagine synthetase?
L-asparaginase performs hydrolysis and produces L-aspartate and ammonia. Asparagine synthetase participates in L-asparagine synthesis. Their reaction direction, energy requirements, structures, and biological roles are different.
Does adding more enzyme always improve food processing?
No. Dose must be evaluated together with substrate availability, mixing, contact time, temperature, pH, and product quality. Beyond an effective range, more enzyme may not produce a proportional benefit and can increase process cost.
Why measure glutaminase side activity?
Some L-asparaginases can also act on glutamine. The importance of that activity depends on the intended use, so target and competing substrates should be tested separately rather than summarized by one total-activity number.
Can computational prediction replace enzyme activity experiments?
No. Computational tools can narrow candidate space, propose mutation hypotheses, and organize priorities. Experiments still confirm expression, folding, activity, specificity, and stability. Their combination increases the amount of useful information generated in each development round.
Conclusion: Clarify the name, then place performance in context
Understanding an asparagine-converting enzyme begins with identifying the reaction under discussion. For L-asparaginase development, the enzyme name, substrate, assay, and application conditions must be linked. Activity is only the starting point; selectivity, stability, expression, and performance in the intended matrix determine candidate value.
The enzyme mining, function prediction, protein design, and directed evolution capabilities organized through MatwingsVenus™(晓鹜™) can support candidate discovery and experimental planning. Clear task boundaries, comparable assays, and staged validation are what turn an enzyme concept into a reliable development decision.